Survey of Drought and Root Morphology Across Southern Wisconsin Prairies
Article by Lucille J. Wineberg, Department of Botany, University of Wisconsin-Madison
Senior Thesis, Dr. Sara Hotchkiss and Christian Villanueva, May 6, 2026
As early as 1830, Wisconsin was home to 971,000 hectares of prairie. From 1830-1994, prairie loss accelerated, with the majority of the loss caused by European settlements and later urban and agricultural development, reducing prairie cover by 99.9% and leaving the state with roughly 4000 hectares (Samson and Knopf, 1994; Askins et al., 2007). Despite their decline/degradation, prairies remain extremely important in supporting local biodiversity and the environment. Protected and managed ecosystems, such as reconstructed prairies, have positive effects on biodiversity, which then provide ecosystem services by keeping water clean, producing food and regulating the climate (Woodley et al., 2015).
Since 2021, Wisconsin has endured an abnormal increase in level of drought severity throughout the state. At points during the summer of 2023, 81% of the state was experiencing drought, with 12.2% in extreme drought (level D3). Moreover, much of the drought was concentrated in southern Wisconsin, where prairies are prevalent (National Integrated Drought Information System, 2017) (Figure 1).
One of the primary ways drought affects grassland ecosystems is by lowering the nutrient availability within the soil. When soil is re-moistened after a prolonged dry period, microbes are killed and carbon and nitrogen mineralization increases, making nutrient uptake more difficult (Vries et al., 2016).
Nutrient absorption is mainly controlled by the underground architecture of the plant, specifically their root systems. Plant root structure is divided into two broad categories: taproot systems and fibrous root systems (Figure 2). While fibrous roots tend to spread and stay closer to the surface, taproots probe deeper into the soil. Typically, taproots serve to gain more water access for the plant, and fibrous roots increase nutrient uptake (Anbarasan and Ramesh, 2021). We expect that taproots will be more prevalent in dry prairies, and fibrous roots will be more prevalent in wet prairies, but given climatic shifts, changes in taproot and fibrous root dominance are still unknown.
To track these potential underground shifts on a broader scale, we are exploring aboveground remote sensing technologies. Advances in satellite and aerial imagery quality and availability have allowed for additional opportunities to monitor landscape conditions, especially with the Normalized Difference Vegetation Index (NDVI), a remote sensing derived vegetation index which measures an ecosystem’s health based on the difference between the red and near-infrared light being reflected from the ground (NASA Earthdata, 2024). The NDVI scale ranges from -1 to 1, with the healthier photosynthesizing plants receiving a higher score. Previous studies have found that NDVI varies based on wetland type and condition but is typically lower because the water interferes with the signal (Taddeo et al., 2019). But, in a drought with limited water resources, these wet prairie areas may have a healthier NDVI value due to more access to water and less visible water, while dry prairies will hold a lower value.
This study examines plant species composition within the different types of prairies of southern Wisconsin, comparing root morphology to understand how environmental changes have affected relative frequency of plant morphology types in prairies. We hypothesize that wet prairies will exhibit a higher ratio of fibrous roots to taproots, while dry prairies will show the opposite pattern. We further expect reconstructed prairies to have higher NDVI due to active management, along with wet prairies because of higher moisture.
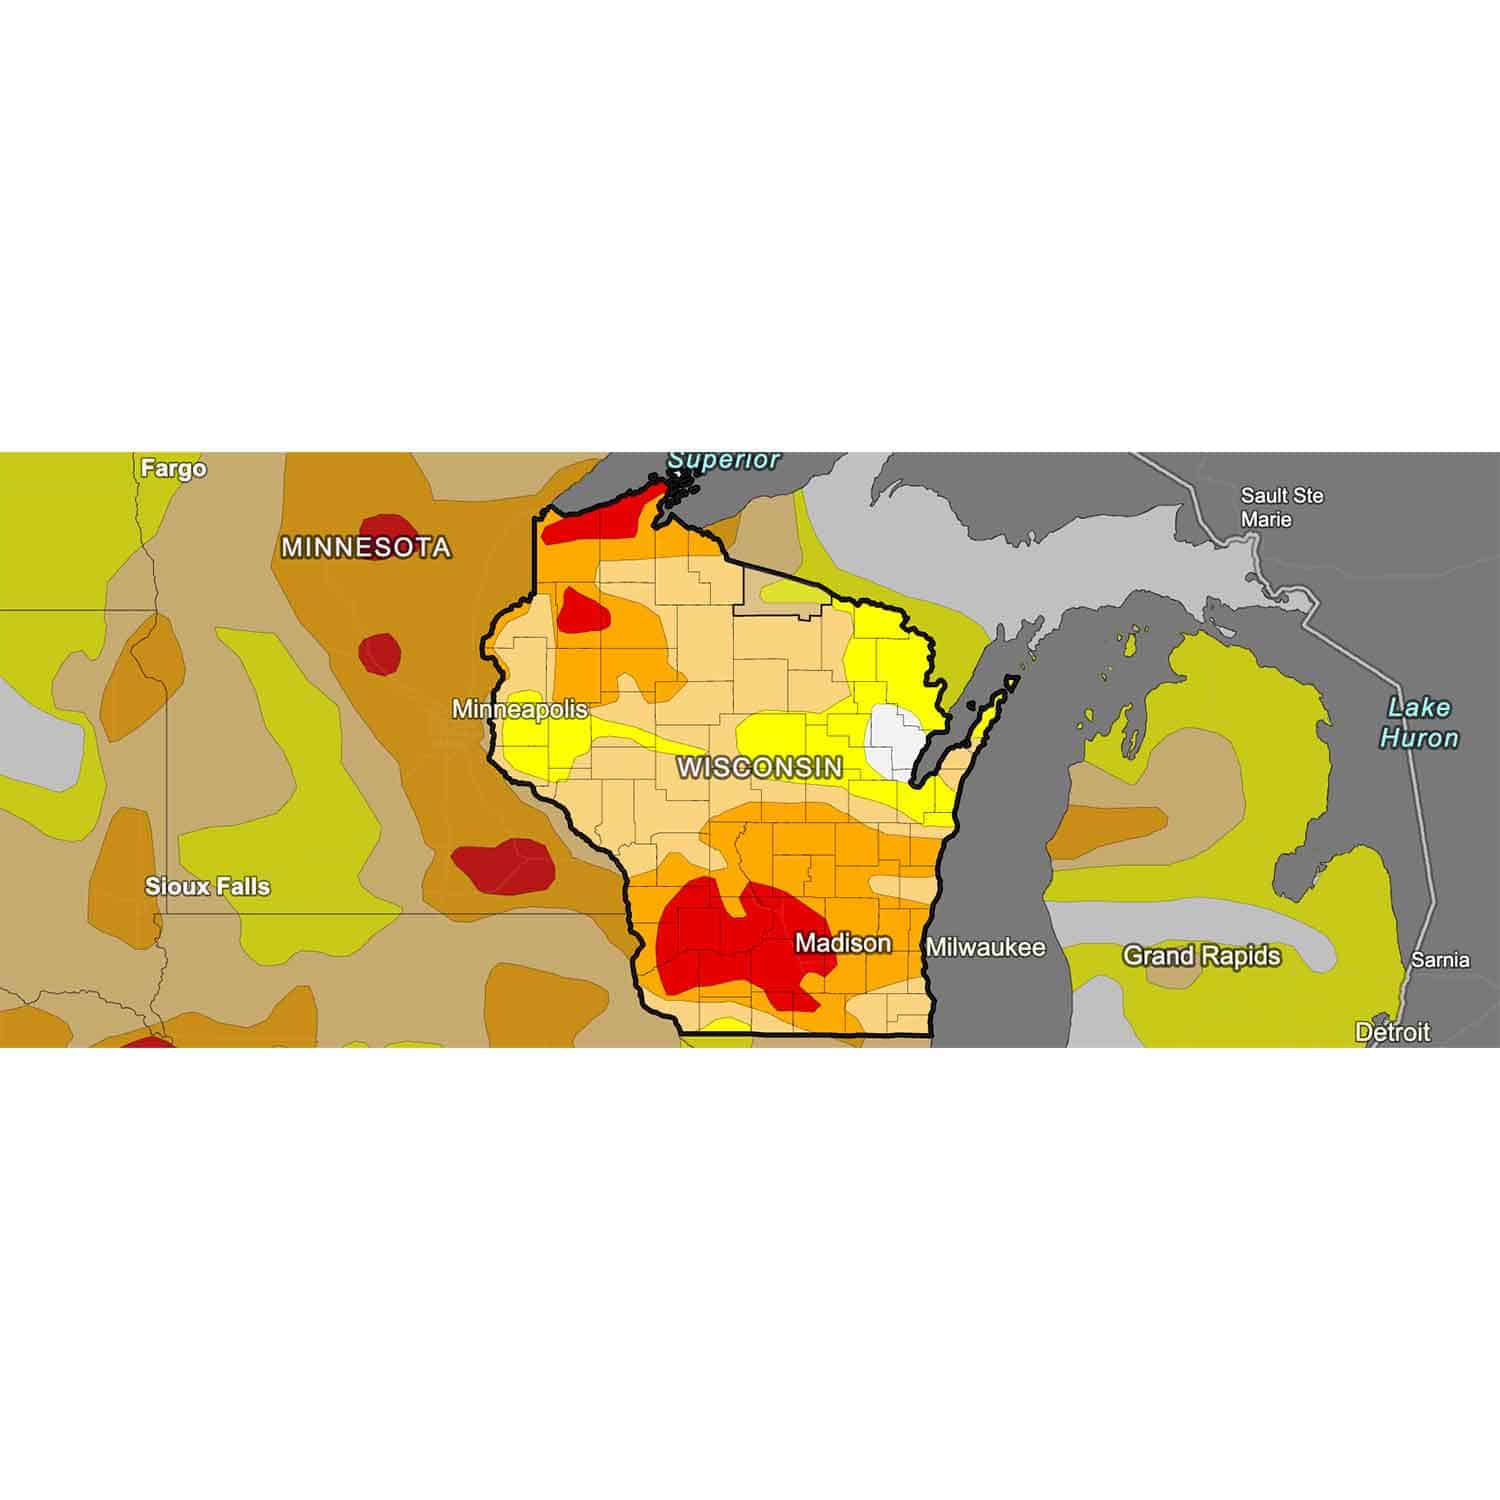
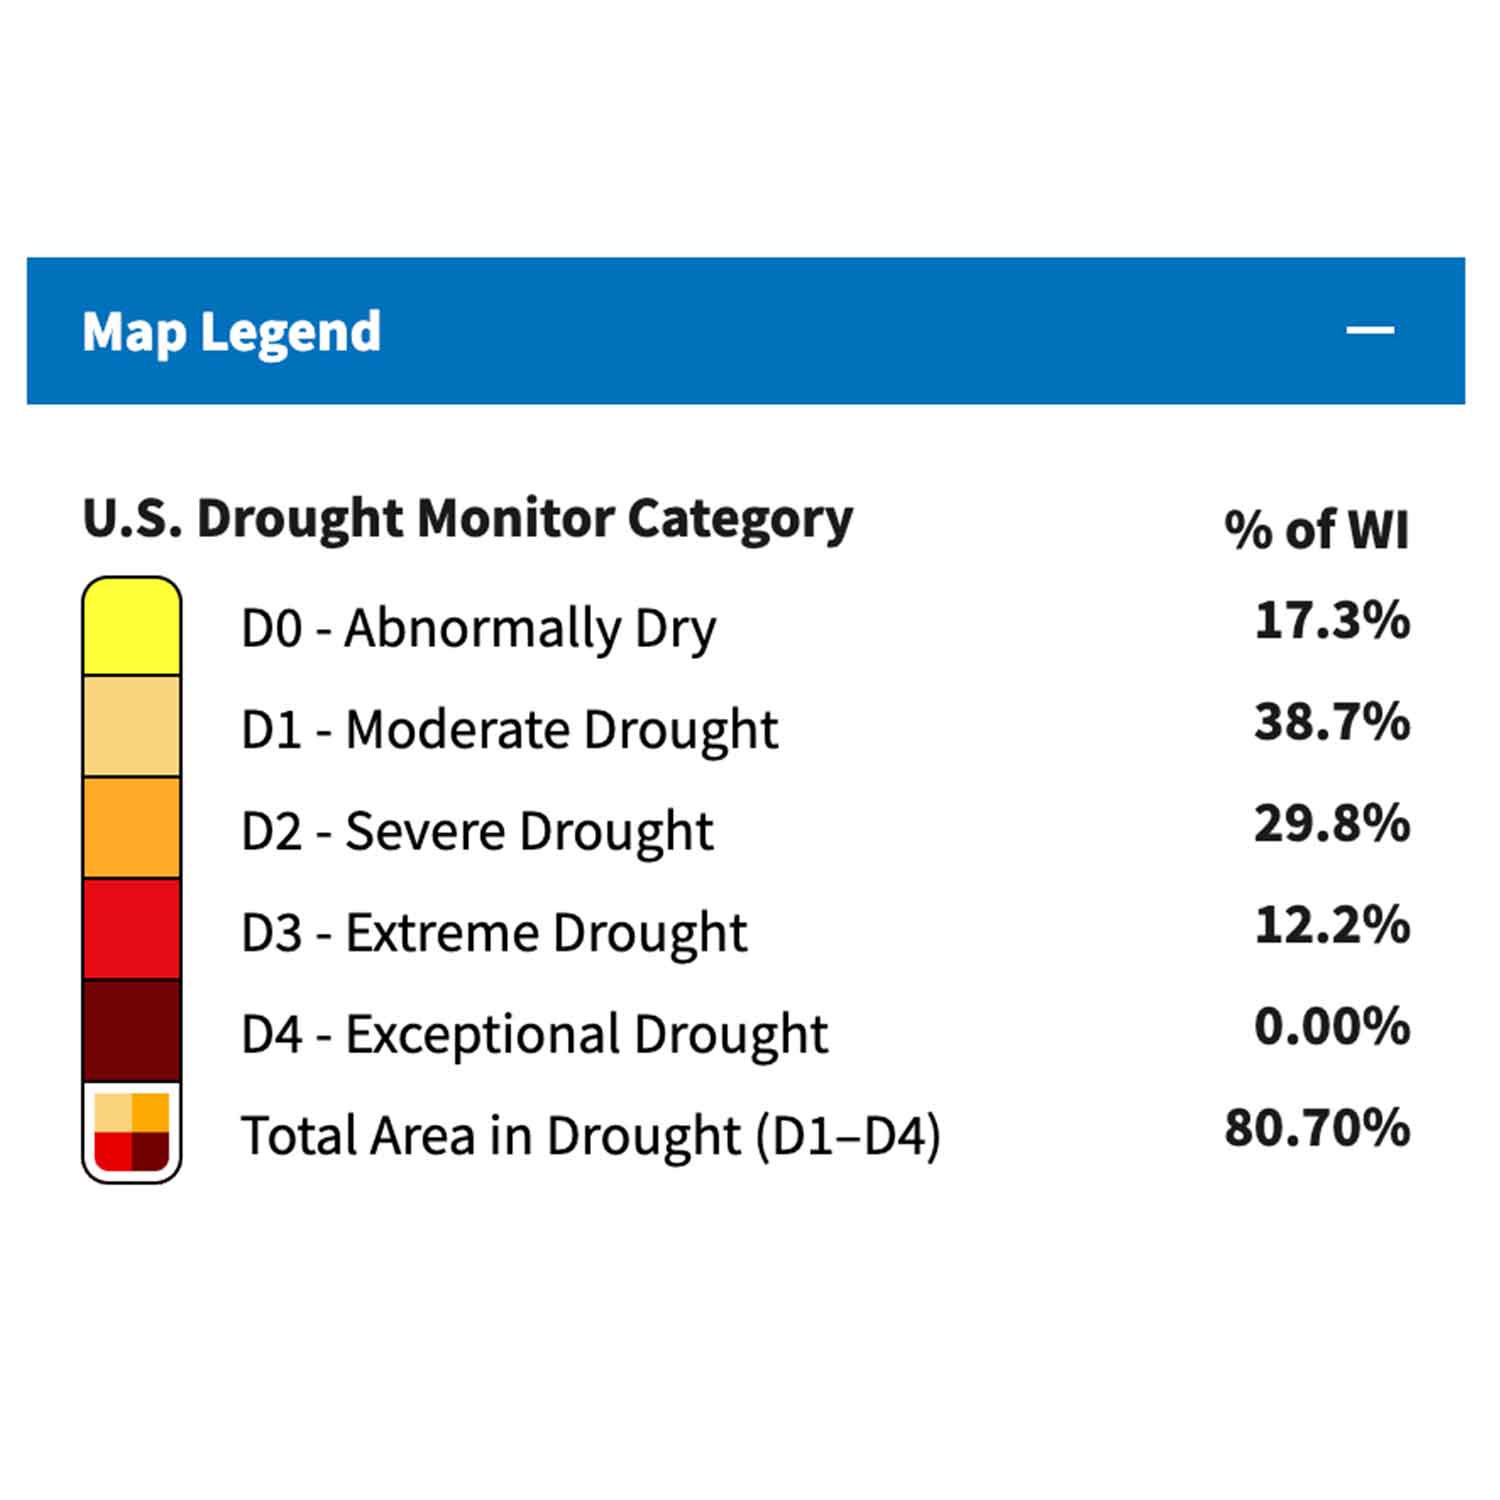
Figure 1. Wisconsin drought levels on August 1, 2023 (National Integrated Drought Information System, 2017).
Methods
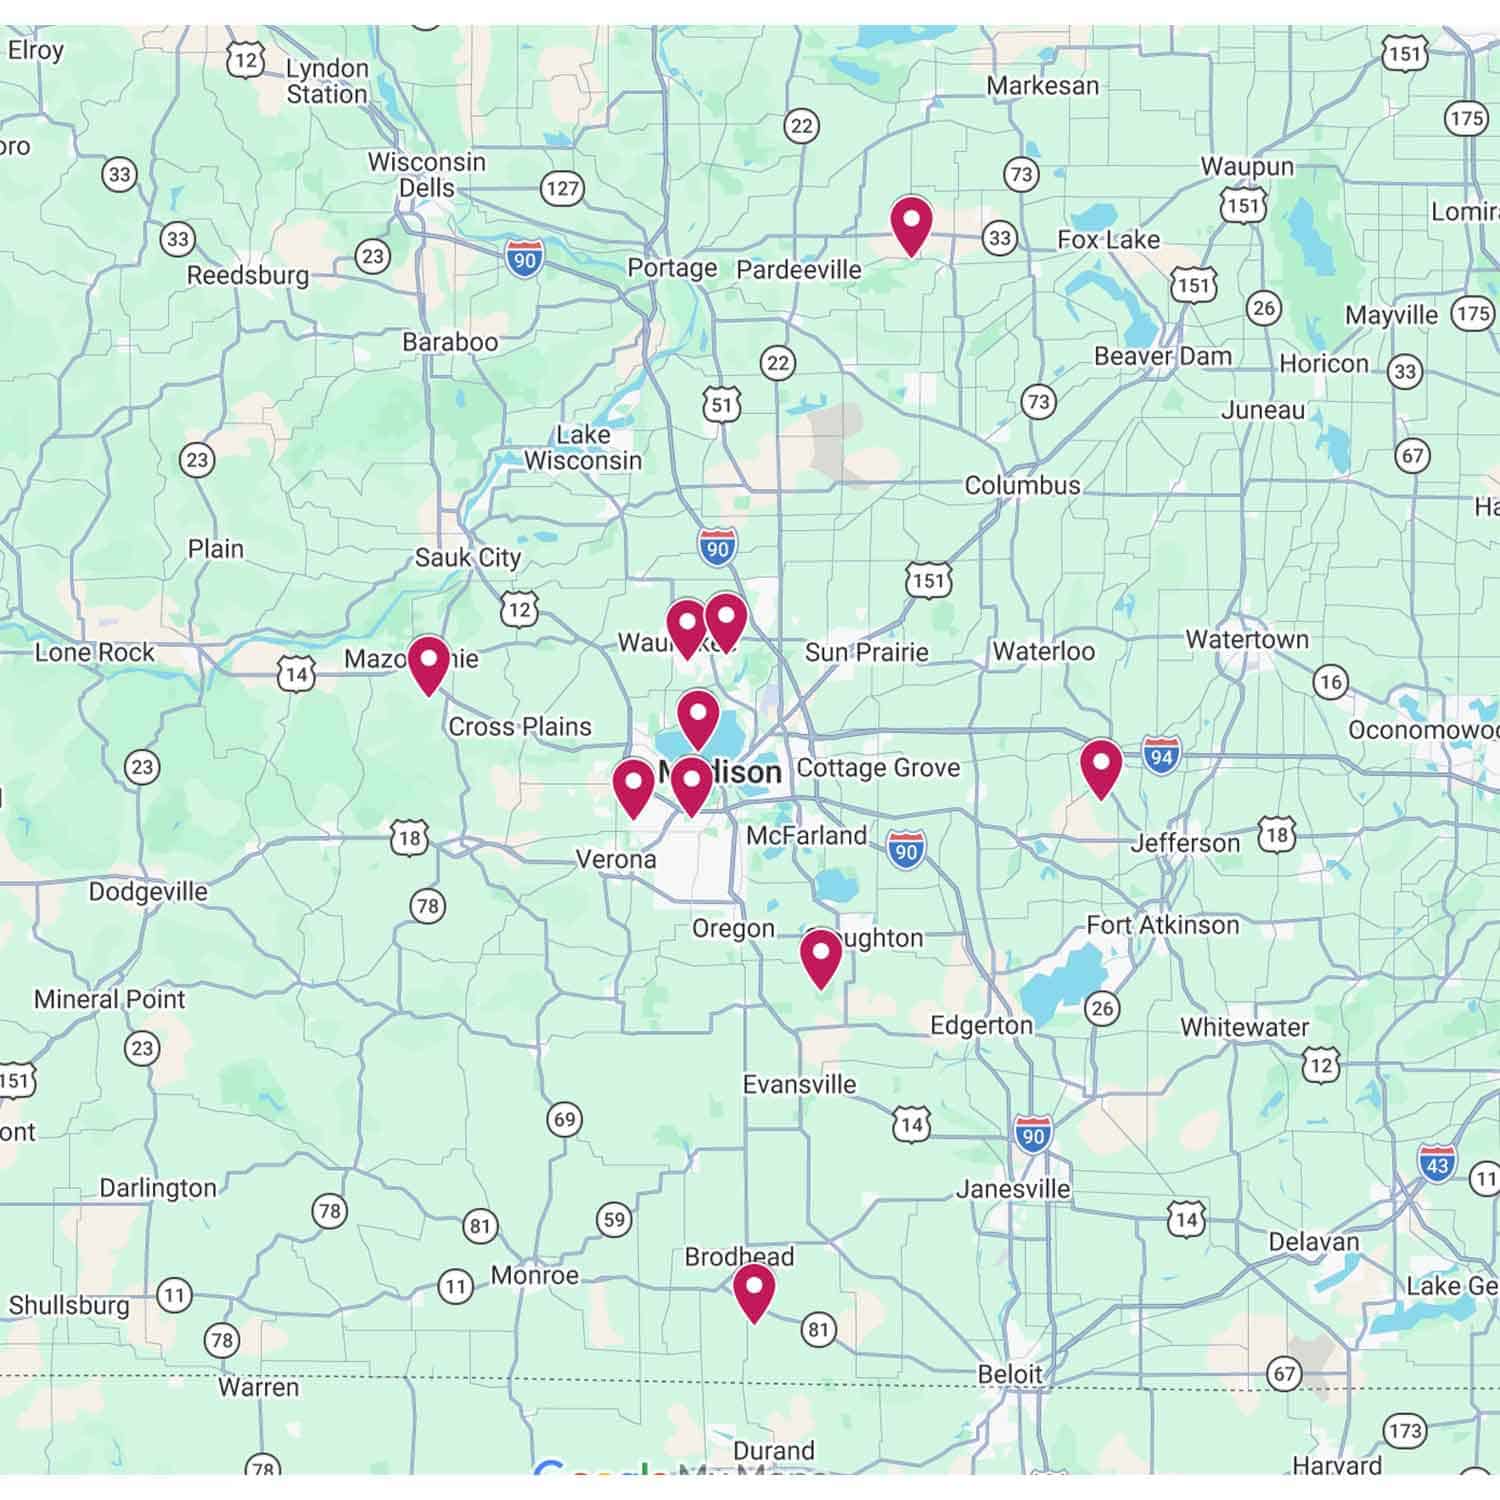
The data collection portion of this study was conducted from June 2025 to November 2025, surveying 11 sites in southern Wisconsin (Figure 3). Four of the sites sampled were characterized as “dry prairies” based on their historic soil and species composition (UW-Madison Arboretum pers. com.; Lakeshore Nature Preserve, n.d.; Wisconsin Department of Natural Resources, n.d.), with another four labeled as “wet prairies,” one “mixed reconstructed”—a reconstructed site with intermediate soil—and two “dry reconstructed.” At each site, 0.5 meter by 0.5 meter quadrats were taken at randomized points throughout the selected area, with between 10–30 quadrats per site, predetermined depending on site size.
Within each quadrat, we measured the percent cover of each species, including a separate category for any bare ground or foliage. We also noted soil moisture, composition, and if there was a slope within each quadrat. We categorized each species into their root types by gathering information from Illinois Wildflowers (Hilty, 2017), and then comparing that information to photographed specimens found on the Wisconsin State Herbarium Database (Wisconsin State Herbarium, n.d.), and divided the species into taproot or fibrous root.
Later, we obtained the 2025 precipitation data for each site from the United States Department of Agriculture (USDA, 2025). We also gathered surface reflectance values from the most recent USDA National Agriculture Imagery Program survey in 2022 (USDA, 2022) and used QGIS to calculate the NDVI for each site. To analyze the data, we used an Analysis of Variance (ANOVA) to compare NDVI to site type and root type to site type.
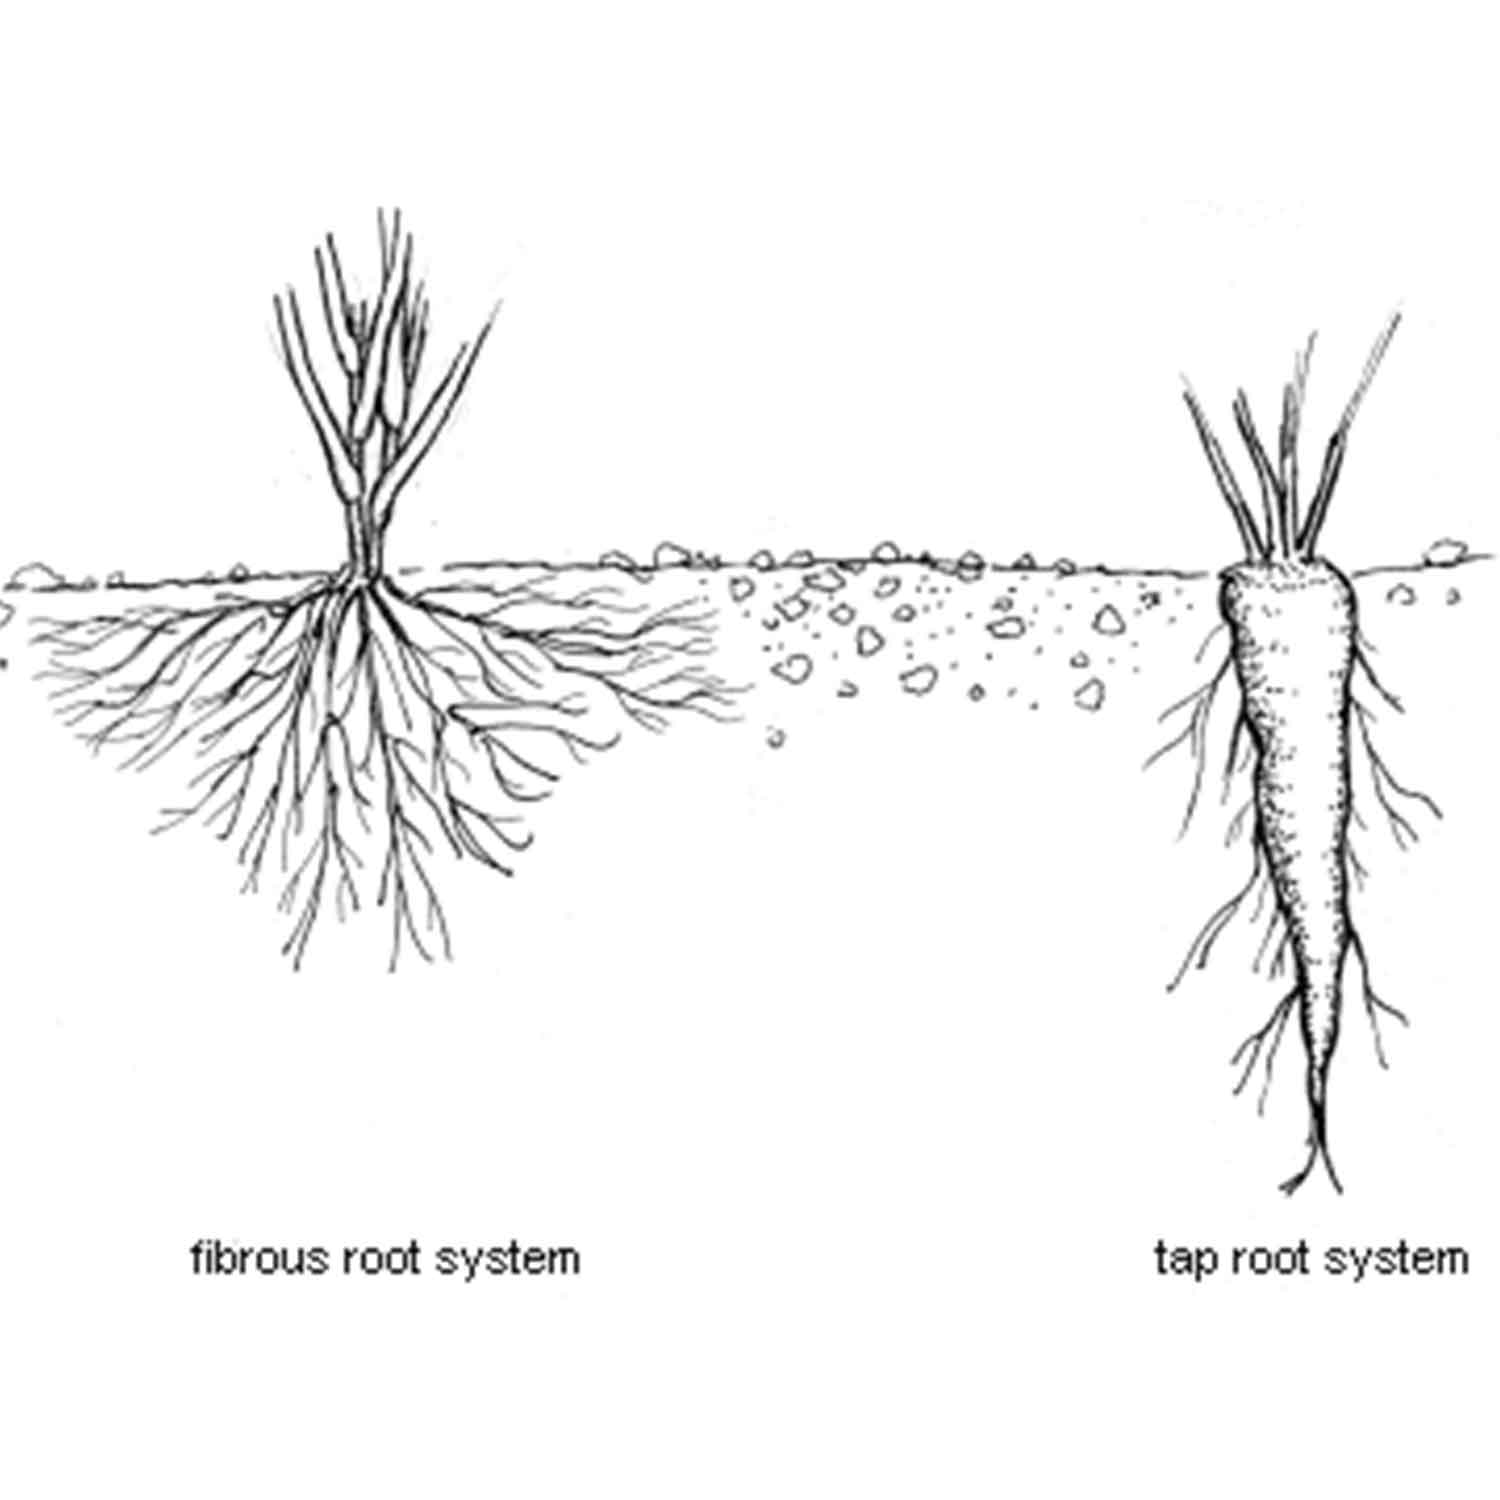
Left: Figure 2: Illustration of root morphology types (National Garden Association, n.d.).
Right: Figure 3: Map of the 11 field sites surveyed. Bolz prairie had two separate sites, on one point.
Results
Over the six months of data collection, we surveyed 11 prairie sites, including four wet prairies, four dry prairies, two dry reconstructed prairies and one mixed reconstructed prairie, observing 164 plant species across all sites. The difference in root-morphology-type percentage was significant (p-value < 0.000001, f statistic of 13.496825), with the highest percent of taproot species in dry reconstructed prairies, closely followed by dry prairies (Figure 4), supporting our hypothesis that we would observe higher fibrous to taproot ratios in wet prairie environments.
While we initially expected wet and reconstructed prairies to have higher NDVI values, there was no significant difference in the NDVI between different site types (p = 0.7816, f = 0.0879), but overall dry reconstructed, mixed reconstructed, and wet prairies held higher values compared to dry prairies (Figure 5).
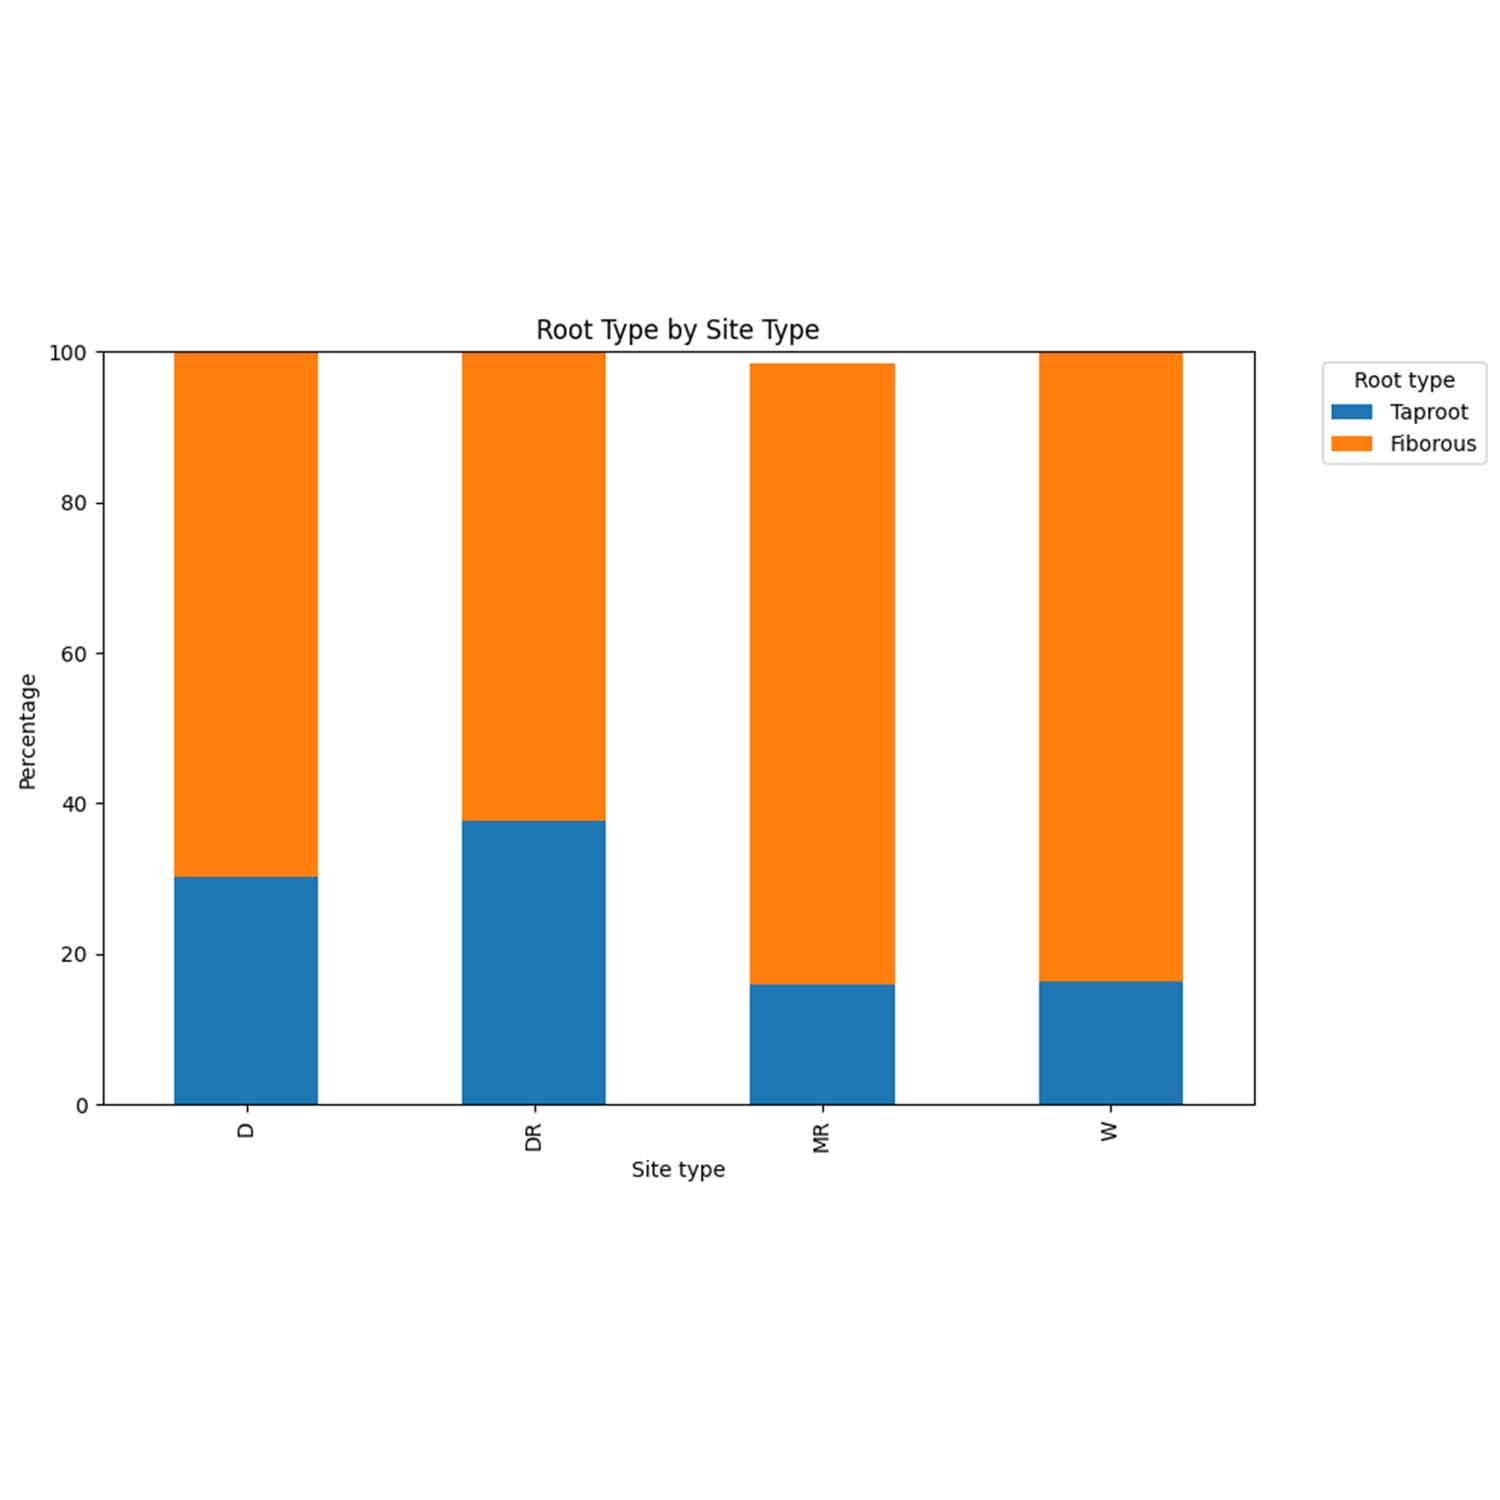
Figure 4: Stacked bar chart of root morphology type by site type classification.
D=Dry Prairies, DR=Dry Restored, MR=Mixed Restored, W=Wet Prairies
Discussion
To determine whether or not prairies respond differently to drought, we tested the Normalized Difference Vegetation Index (NDVI) and percent of individuals with taproot/fibrous root systems at each site. We found no statistically significant difference in NDVI between the different site types, however a marginal difference was noted between sites, specifically the reconstructed prairies (both dry and mixed) held the highest NDVI, closely followed by wet prairies, while dry prairies had the lowest. While wet prairies were deemed “healthier” according to the higher 2022 NDVI value, they had a significantly larger percentage of invasive species, meaning that while these ecosystems have a high biomass, they are functionally less resilient. A large number of the wet prairie sites were covered with Phalaris arundinacea (Reed Canary Grass), a common invasive plant throughout North America (Martina and von Ende, 2013). From observation, P. arundinacea had almost completely overwhelmed any native flora within several individual quadrats.
The root type overall was dominated by fibrous roots, with taproots reaching their maximum share at dry and dry reconstructed prairies (Figure 4), which agrees with the initial hypothesis. However, P. arundinacea has fibrous roots, likely largely influencing the root type percentage.
In comparing the prairie types, Wisconsin’s wet prairies had a high amount of biomass, but were highly infiltrated by P. arundinacea, indicating a lower functional resilience. In the dry prairies, there was a higher species richness and a higher percentage of species with taproots. In reconstructed prairies, there was a higher NDVI and species richness, suggesting success in restoration efforts. In flooded conditions, P. arundinacea is known to do well, explaining why its presence in wet prairies was so apparent. P. arundinacea has been reported to stay relatively healthy in drought conditions, so long as its roots have some sort of contact with water (Kemp & Culvenor, 1994).
Our findings demonstrate the importance of understanding how shifts in the climate affect ecosystem health, even if not entirely apparent at first, which is especially important considering the anticipated climate changes southern Wisconsin is expected to face. However, there is much more to be done to grasp a full understanding of changes within prairie ecosystem remnants in Wisconsin. Considering the varied lifespans of prairie plants and climatic shifts in Wisconsin, long term studies could analyze the species’ turnover in different types of prairies. This would help us understand how these prairies have changed, and apply that to learn how they are expected to change. While we now understand where taproots are more prominent, further research in the depth of the roots could help researchers know what species may be more sensitive to droughts of particular magnitudes, and which are more likely to withstand dry conditions. Overall, the information gained from this study will enhance our understanding on how drought impacts different types of prairie ecosystems, vegetative health, and overall biodiversity, helping us protect these sensitive ecosystems.
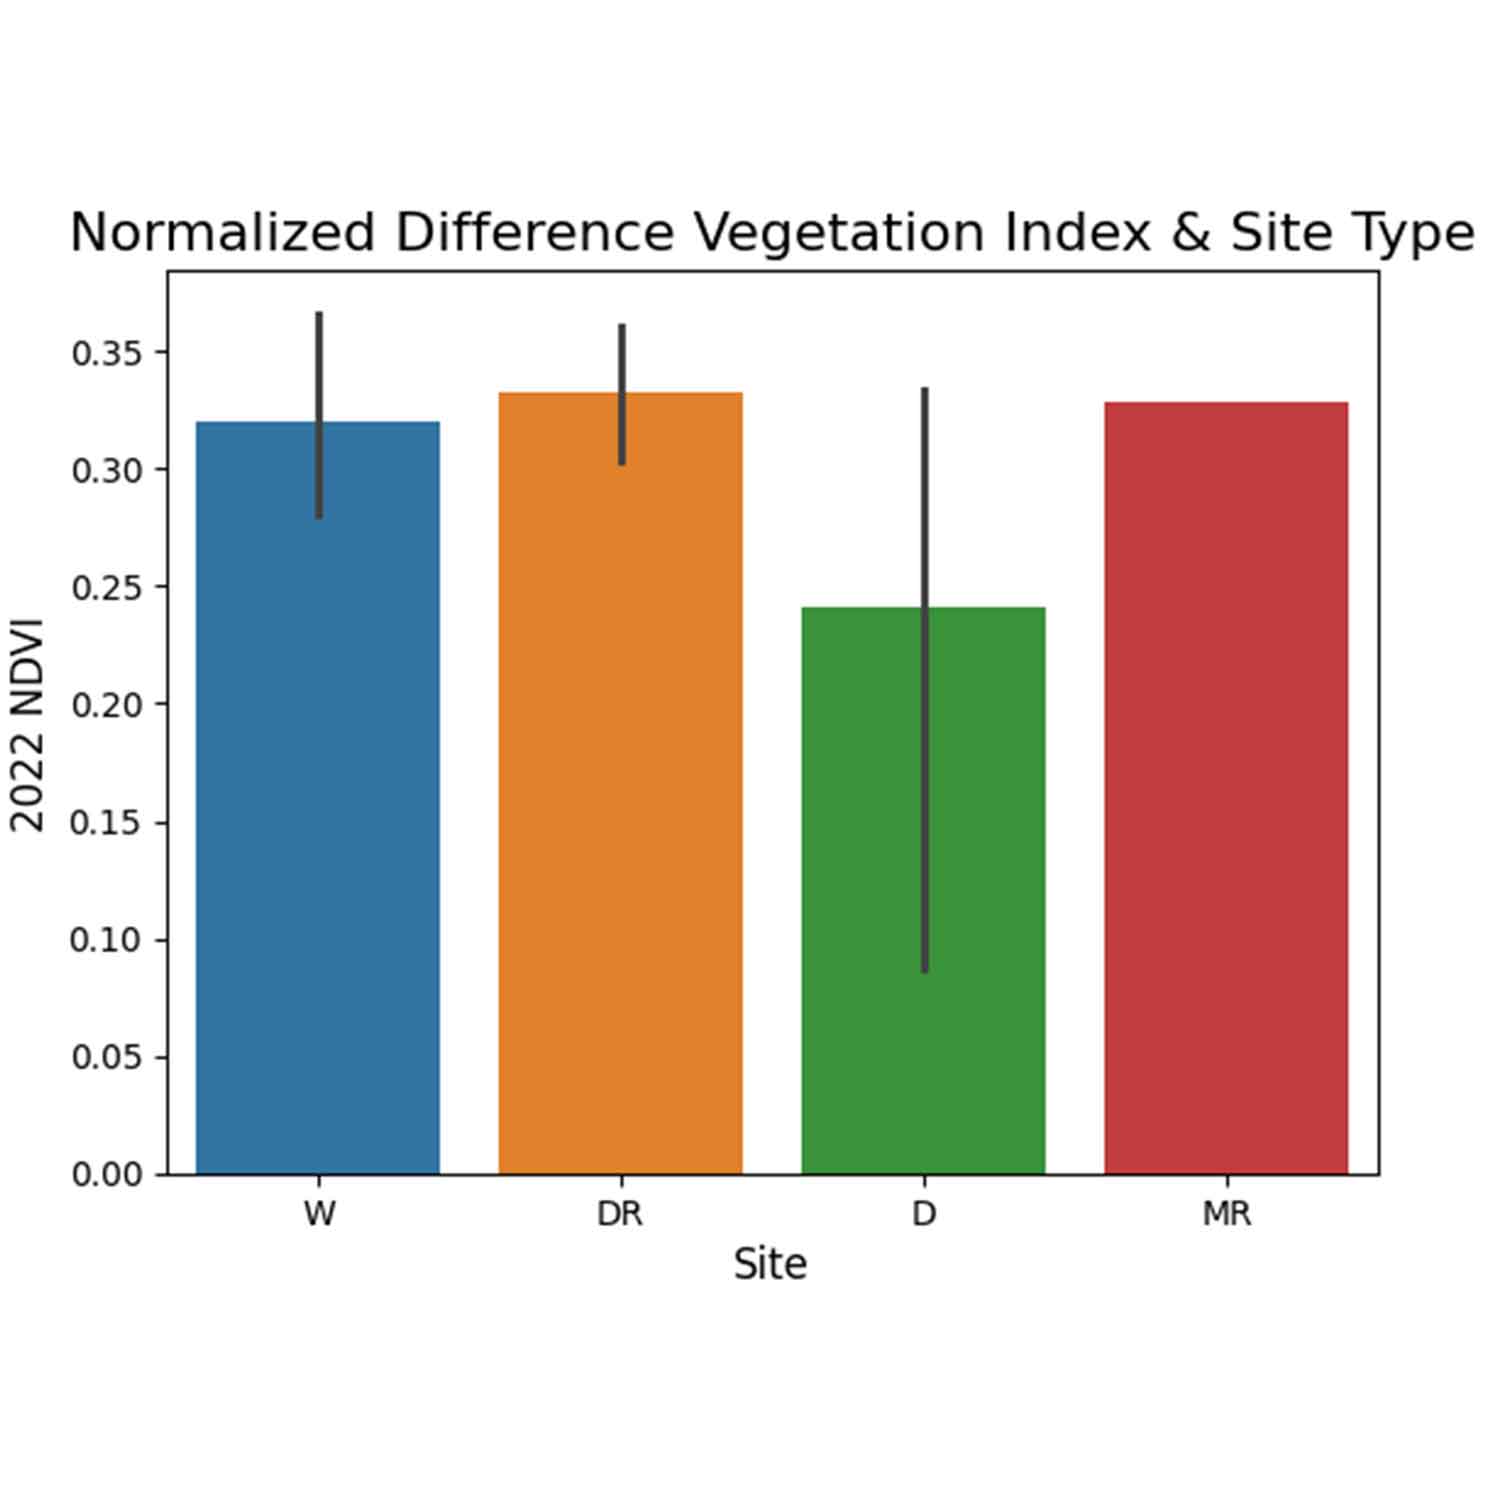
Figure 5: Bar chart of NDVI compared to site type.
D=Dry Prairies, DR=Dry Restored, MR=Mixed Restored, W=Wet Prairies
Acknowledgements
This project was supported and funded by the UW-Madison Botany Department. I would like to thank Christian Villanueva, Dr. Sara Hotchkiss and Mark Connolly for the consistent support, mentorship, and insightful feedback through this process.
References
Adams, C. R., & Galatowitsch, S. M. (2005). Phalaris arundinacea (reed canary grass): Rapid growth and growth pattern in conditions approximating newly restored wetlands. Ecoscience, 12(4), 569–573. https://doi.org/10.2980/i1195-6860-12-4-569.1
Anbarasan, S., & Ramesh, S. (2021, February). The Role of Plant Roots in Nutrient Uptake and Soil Health. Plantarc.com; Plant Science Archives. https://plantarc.com/the-role-of-plant-roots-in-nutrient-uptake-and-soil-health/
Askins, R. A., Chávez-Ramírez, F., Dale, B. C., Haas, C. A., Herkert, J. R., Knopf, F. L., & Vickery, P. D. (2007). Conservation of Grassland Birds in North America: Understanding Ecological Processes in Different Regions: “Report of the AOU Committee on Conservation.” Ornithological Monographs, 64, iii–46. https://doi.org/10.2307/40166905
Bai, Y., & Cotrufo, M. F. (2022). Grassland soil carbon sequestration: Current understanding, challenges, and solutions. Science, 377(6606), 603–608. https://doi.org/10.1126/science.abo2380
Hilty, J. (2017). Illinois Wildflowers. Illinoiswildflowers.info. https://www.illinoiswildflowers.info/
Kemp, D. R., & Culvenor, R. A. (1994). Improving the grazing and drought tolerance of temperate perennial grasses. New Zealand Journal of Agricultural Research, 37(3), 365–378. https://doi.org/10.1080/00288233.1994.9513074
Kercher, S. M., Carpenter, Q. J., & Zedler, J. B. (2004). Interrelationships of Hydrologie Disturbance, Reed Canary Grass (Phalaris arundinacea L), and Native Plants in Wisconsin Wet Meadows. Natural Areas Journal, 24(4), 316–325. JSTOR. https://doi.org/10.2307/43912343
Lakeshore Nature Preserve. (n.d.). Biocore Prairie. Lakeshore Nature Preserve. https://lakeshorepreserve.wisc.edu/visit/places/biocore-prairie/
Martina, J. P., & von Ende, C. N. (2013). Increased spatial dominance in high nitrogen, saturated soil due to clonal architecture plasticity of the invasive wetland plant, Phalaris arundinacea. Plant Ecology, 214(12), 1443–1453. JSTOR. https://doi.org/10.2307/24553725
NASA Earthdata. (2024, September 30). Normalized Difference Vegetation Index (NDVI) | NASA Earthdata. NASA Earthdata. https://www.earthdata.nasa.gov/topics/land-surface/normalized-difference-vegetation-index-ndvi
National Garden Association. (n.d.). Roots as Anchors. Garden.org. https://garden.org/courseweb/course1/week1/page8.htm
National Integrated Drought Information System. (2017). Historical Data and Conditions. Drought.gov. https://www.drought.gov/historical-information?dataset=0&selectedDateUSDM=20230801&state=Wisconsin
Samson, F., & Knopf, F. (1994). Prairie Conservation in North America. BioScience, 44(6), 418–421. https://doi.org/10.2307/1312365
Schulte, L. A., Anna Lynn MacDonald, Niemi, J., & Helmers, M. J. (2016). Prairie strips as a mechanism to promote land sharing by birds in industrial agricultural landscapes. Agriculture, Ecosystems & Environment, 220, 55–63. https://doi.org/10.1016/j.agee.2016.01.007
Taddeo, S., Dronova, I., & Depsky, N. (2019). Spectral vegetation indices of wetland greenness: Responses to vegetation structure, composition, and spatial distribution. Remote Sensing of Environment, 234(111467). https://doi.org/10.1016/j.rse.2019.111467
Tresenriter, L., Griffin, J., Hanauer, K., Lowe, B., Fry, O., Stout, S., Johnson, B., & Brooke, J. (n.d.). Reed Canary Grass Control. https://www.purdue.edu/fnr/extension/wp-content/uploads/2025/04/FNR-648ReedCanarygrassADA-final-comp2.pdf
USDA. (2022). National Agriculture Imagery Program Hub Site. Naip-Usdaonline.hub.arcgis.com. https://naip-usdaonline.hub.arcgis.com/
USDA. (2025). Snowpack and Precipitation Index Maps | Natural Resources Conservation Service. Natural Resources Conservation Service. https://www.nrcs.usda.gov/programs-initiatives/sswsf-snow-survey-and-water-supply-forecasting-program/snowpack-and
Vries, F., Brown, C., & Stevens, C. (2016). Grassland species root response to drought: consequences for soil carbon and nitrogen availability. Plant and Soil, 409(1/2), 297–312. https://doi.org/10.2307/44245232
Weaver, J. E., & Albertson, F. W. (1943). Resurvey of Grasses, Forbs, and Underground Plant Parts at the End of the Great Drought. Ecological Monographs, 13(1), 63–117. https://doi.org/10.2307/1943590
Weaver, J. E., Stoddart, L. A., & Noll, Wm. (1935). Response of the Prairie to the Great Drought of 1934. Ecology, 16(4), 612. https://doi.org/10.2307/1932592
Wisconsin Department of Natural Resources. (n.d.). Protecting Wisconsin’s Biodiversity – Natural Communities. Apps.dnr.wi.gov. https://apps.dnr.wi.gov/biodiversity/Home/index/communities
Wisconsin State Herbarium. (n.d.). Online Virtual Flora of Wisconsin Home. Wisflora.herbarium.wisc.edu. https://wisflora.herbarium.wisc.edu/index.php
Woodley, S., MacKinnon, K., McCanny, S., Pither, R., Prior, K., Salafsky, N., & Lindenmayer, D. (2015). Managing Protected Areas for Biological Diversity and Ecosystem Functions (G. L. Worboys, M. Lockwood, A. Kothari, S. Feary, & I. Pulsford, Eds.). JSTOR; ANU Press. https://www.jstor.org/stable/j.ctt1657v5d.28
About The Prairie Enthusiasts
The Prairie Enthusiasts is an accredited land trust that seeks to ensure the perpetuation and recovery of prairie, oak savanna, and other fire-dependent ecosystems of the Upper Midwest through protection, management, restoration, and education. In doing so, they strive to work openly and cooperatively with private landowners and other private and public conservation groups. Their management and stewardship centers on high-quality remnants, which contain nearly all the components of endangered prairie communities.